

1. Introduction
Mung bean, scientifically known as Vigna radiata (L.) R. Wilczek, belongs to the family Fabaceae and is categorized within the subfamily Faboideae. It is part of the genus Vigna, specifically identified as the species V. radiata (L.) R. Wilczek. The genus Vigna is typically found in warm-temperate and tropical regions worldwide (Swamy, 2023). This species is considered agronomically important due to its ability to thrive in poor soils, short reproductive period, efficient nitrogen fixation, and versatility across a range of environmental conditions (Zheng et al., 2023). In the Philippines where mung bean is locally known as monggo, it is a staple crop primarily cultivated for human consumption and may also serve as an important source of income for farmers (Pattung et al., 2023).
The crop is appreciated not just for its adaptability in various agricultural settings but also for its abundant nutritional benefits and is positioned as a viable solution for improving food and nutritional security. Despite the crop’s capacity to enhance sustainable agriculture and improve local livelihoods, the Philippines continues to rely significantly on imported mung beans to satisfy domestic demand. In 2022, the nation imported approximately 50,000 metric tons of mung beans, valued at around $40 million, highlighting the disparity between domestic output and consumption. In 2021, local production satisfied merely 27% of overall pulse consumption (Lagare, 2023). Such imbalance underscores the urgent need to advocate for the localized agricultural production of high-potential native plant variety.
One such variety in the Philippines is the yellow mung bean (YMB, NSIC Mg 22). Released in 2020, this variety is distinguished by its glossy yellow seeds, which weigh between 5.9 and 6.6 g per 100 seeds. It exhibits moderate resistance to various diseases, such as Cercospora leaf spot and rust. The seeds are nutritionally rich, containing approximately 24.7% crude protein and 0.6% crude fat (Bureau of Plant Industry, n.d.). The focus on YMB variety in this study is driven by its agricultural potential and its unique yet underutilized biochemical profile. While the macronutrient content of green varieties and other legumes are often well documented, comprehensive research detailing the nutritional and functional attributes of local mung bean varieties like YMB remains insufficient.
Emerging research indicates that the seed coat color is a major determinant of a seed’s phytochemical composition (Wu et al., 2026). However, current studies lack data regarding their antioxidant and phenolic profiles of YMB. These bioactive compounds are directly linked to human health, as these antioxidants play a critical role in neutralizing cellular oxidative stress and reducing the risk of chronic diseases (Hou et al., 2019). Because the nutritional and biochemical profile of legumes, such as mung beans, can differ markedly (Dahiya et al., 2013) due to variables like genetics, soil conditions, climate, and agricultural methods, localized research is essential to fully utilize these crops as functional foods.
To support local cultivation efforts and explore the market potential of native varieties, this study focused on the comprehensive analysis of locally grown YMB. Specifically, it aimed to determine its mineral content, proximate composition, and amino acid profile, as well as to assess its antioxidant activity. It was hypothesized that locally grown YMB would contain nutritionally significant levels of protein, essential amino acids, and selected minerals, along with measurable antioxidant activity. The findings may contribute valuable data that inform breeding programs, nutritional labeling, and the promotion of locally grown mung beans as a nutritious and functional food source.
2. Materials and methods
The YMB NSIC Mg 22 variety used in this study was obtained from the Bureau of Plant Industry-La Granja National Crop Research, Development, and Production Support Center (BPI-LGNCRDPSC), located in La Carlota City, Negros Occidental, Philippines. The identity of the sample was authenticated by Niña Kathryn G. Alfeche, M.Sc., Curator, University of Santo Tomas Herbarium.
The bulk sample (whole beans) was transferred into a rotary mixer and homogenized three times for 10 min each. After mixing, representative subsamples were collected for laboratory analyses, including proximate composition, mineral content, amino acid profiling, and antioxidant assays. Prior to analysis, the samples were stored in the refrigerator and subsequently pulverized before weighing. All analyses except for antioxidant assays were reported on a wet weight (as received) basis.
Ultrapure water was utilized throughout all experimental procedures. Analytical-grade reagents were procured from Merck (Darmstadt, Germany), Sisco Research Laboratories (Maharashtra, India), and Sigma-Aldrich (Buchs, Switzerland). A Certified Reference Material (AccuStandard, New Haven, CT, USA) with a stated purity of 99.99% was used in mineral analysis.
The method used for moisture determination follows the AOAC method 964.22 (AOAC International, 2023). A sample weighing about 2 ± 0.001 g was placed in a pre- weighed aluminum dish and dried at 70°C for 2 h using a convection oven (VO400 Vacuum Oven, Memmert, Schwabach, Germany). The difference in weights before and after drying represents the moisture content.
Kjeldahl method with an automated FOSS DT 220 Digestor and Kjeltec 8100 Distillation Unit (FOSS Analytical, Hillerød, Denmark) was used in the determination of crude protein. Around 1 ± 0.001 g of the sample was digested at 420°C for 2 h. The resulting distillate was back-titrated with 0.25 N HCl. Crude protein in the sample was calculated by multiplying the total nitrogen content by a conversion factor of 6.25 (Hall and Schönfeldt, 2013).
Crude fat was analyzed using acid hydrolysis followed by a gravimetric method. A 2 ± 0.001 g sample was hydrolyzed using HCl prepared by mixing concentrated HCl and water at a 25:11 (v/v) ratio. Fat was extracted three times using a mixture of petroleum ether and diethyl ether (25:25, v/v). The solvent was evaporated in a water bath, and the extraction flask was dried in an air oven, cooled, and repeatedly weighed until a constant weight was reached.
A gravimetric method was used in the analysis. Approximately 1 ± 0.001 g of the sample in a crucible was charred, cooled, and weighed before ashing in a muffle furnace (Daihan Electric Muffle Furnace, Wonju, Korea). The temperature was gradually increased to 550°C and maintained for 8 h until a white or nearly white residue was obtained.
The total carbohydrate content was calculated by difference according to Dudasova (2025), as follows:
The total energy content was determined through the results of the proximate analysis by summing the amounts (g/100 g) of crude protein, crude fat, and total carbohydrates, and multiplying each by its respective Atwater conversion factors: 4 kcal/g for protein and carbohydrates, and 9 kcal/g for fat (Ayogu et al., 2022).
Before hydrolysis, cysteine and methionine underwent oxidation to form cysteic acid and methionine sulfone, respectively, to ensure accurate quantification. As tyrosine is susceptible to destruction during oxidation, it was determined from hydrolysates of unoxidized samples. All other amino acids were quantified from either oxidized or unoxidized samples, as appropriate. Oxidation was carried out using a performic acid/phenol mixture, followed by the addition of sodium metabisulfite to decompose any excess oxidizing reagent. Following this, both the oxidized and unoxidized samples underwent hydrolysis using 6N HCl. The separation of components was through ion-exchange chromatography and quantification through a reaction with ninhydrin, employing photometric detection at 570 nm (440 nm specifically for proline). The flow in the buffer and ninhydrin lines was provided by pumps having a flow stability of ± 0.5% in the period covering both the standard calibration run and the analysis of the sample.
A sample weighing 10.0 ± 0.1 g was measured with an analytical balance (Mettler Toledo ME104E, Greifensee, Switzerland) in a 50 mL crucible. The sample underwent charring on a hot plate and subsequent incineration in a muffle furnace at 550°C for 16 h, or until a grayish-white ash was obtained. After incineration, the sample was dissolved in 10 mL of 6 N HCl and placed on a hot plate to aid dissolution. The digested sample was transferred to a volumetric flask and diluted to 50 mL using ultrapure deionized water. The digestate was filtered with Whatman filter paper no. 1 prior to readings.
Digestion blanks were prepared and processed together with the samples from ashing through instrumental reading for quality control. A multi-element standard solution was prepared, and six calibration standards at 0, 2, 4, 6, 8, and 10 ppm were generated to establish calibration curves with correlation coefficients (r) of at least 0.99.
The mineral content was quantified using the inductively coupled plasma-optical emission spectroscopy (Agilent 5800-ICP-OES, Agilent Technologies, Santa Clara, CA, USA) using the following wavelengths (nm): Ca (422.673), Fe (259.940), K (766.491), Na (588.995), Zn (Axi-213.857), Cu (Rad-327.395), Mg (Rad-279.553) and Mn (Rad-259.372).
A modified extraction method was followed based on the approach outlined by Wanyo et al. (2016). A 1.00 g portion of the homogenized sample was carefully measured and placed into a centrifuge tube. Subsequently, 10 mL of absolute ethanol was incorporated into the mixture, which was then subjected to vortex mixing. The tube was subsequently placed in a water bath set at 37°C for 1 h. It was shielded from direct light and gently shaken at intervals to aid in the extraction process. After the incubation period, the mixture underwent centrifugation at 2,000 rpm using a benchtop centrifuge (Universal 320 R, Hettich, Tuttlingen, Germany) with the temperature controlled at 20°C for 15 min to yield a clear supernatant.
The analysis was conducted following the methodologies established by Satpute et al. (2012) and Sik et al. (2022), with some modifications. A 0.2 mL of control (absolute ethanol) was pipetted to a clean test tube. Next, 1.5 mL of Folin-Ciocalteu reagent was introduced, and the resulting solution was incubated in a water bath at 22°C for 5 min. Following this, 1.5 mL of 0.57 M sodium carbonate solution was introduced. The reaction mixture was incubated in the dark at 22°C for 90 min. After incubation, the absorbance was measured at 725 nm using a UV-Vis spectrophotometer (UV-1900i, Shimadzu, Kyoto, Japan). This served as the control absorbance (Ac).
Gallic acid standards (16, 42, 84, 148, and 169 mg/L) were prepared and analyzed under identical conditions to construct a calibration curve (R2 ≥ 0.99). Absorbance values were plotted against gallic acid concentrations, and the regression equation was used for quantification.
Sample extracts were analyzed using the same procedure. TPC was expressed as gallic acid equivalents (GAE) per unit dry weight (DW) of sample using the formula:
where:
Gallic Acid Conc. = value from calibration curve in mg/L
Vextract = volume of sample extract used in mL
DF = dilution factor
m = mass of sample used in g
F = conversion factor to convert wet weight to dry weight
The assay was performed following the method by Liao et al. (2012) with modifications. A 1.00 mL aliquot of the control (absolute ethanol) was transferred into a clean test tube. Subsequently, 2.00 mL of DPPH solution was added. The mixture was placed in the dark at room temperature for 30 min to promote the reaction. Following this, absorbance was measured at 517 nm using a UV-Vis spectrophotometer. This served as the control absorbance (Ac).
The DPPH radical scavenging activity of the sample extracts was determined based on the Trolox calibration curve. The results were calculated and expressed as Trolox equivalents (TE) per unit dry weight of the sample (μmol TE/100 g DW).
The assay was adapted from the method of Gohari et al. (2011). A 0.10 mL aliquot of absolute ethanol was transferred into a clean glass vial or test tube, followed by the addition of 3.00 mL of freshly prepared FRAP reagent. The FRAP reagent consisted of a mixture of 5.00 mL of 10 mM 2,4,6-tri(2-pyridyl)-1,3,5-triazine solution, 5.00 mL of 20 mM FeCl3 and 50.00 mL of pH 3.6 acetate buffer (6.20 g sodium acetate trihydrate in 32.00 mL acetic acid diluted to 50.00 mL distilled water). The solution was thoroughly mixed and then placed in a water bath at 37°C for a 10-min incubation period. Measurement of absorbance was carried out at 593 nm using a UV-Vis spectrophotometer. This served as the control absorbance (Ac).
The FRAP values of the sample extracts were calculated using the linear regression equation obtained from the Trolox calibration curve. The results were expressed as TE per unit dry weight of the sample (μmol TE/100 g DW).
The nutritional value of the YMB was assessed based on its percentage adequacy:
The amount of nutrients present per 100 g of sample was calculated and compared against the estimated average requirement (EAR) for adults (19 years and older) of the Philippine Dietary Reference Intakes 2015 (PDRI 2015) (DOST-FNRI, 2017). EAR represents the daily nutrient intake level that satisfies the median needs of healthy individuals within a specific life stage and is used to estimate the intake for a group or population. For nutrients without an EAR value, Adequate Intake (AI) values were used for comparison purposes.
Each chemical analysis was performed independently in triplicate (n = 3). Analysis results were encoded and analyzed using Microsoft Excel 2021 version 2504. All data were reported as mean ± SD.
No statistical tests were performed to compare the study results with literature data, as differences in sample type, analytical methods, and study design prevent direct inferential comparison. Comparisons with previously published values were conducted descriptively to provide context.
3. Results and discussion
The proximate analysis of YMB provides valuable insights into its nutritional profile, highlighting its potential as a significant dietary component. Table 1 summarizes the analyzed parameters, which collectively reflect the overall composition and nutritive value of the legume.
The moisture content of the sample was 7.48 g/100 g, which is within the range typically reported for dried legumes. This value is slightly below the mean moisture content of 9.51 g/100 g reported by Zafar et al. (2023) for mung bean varieties cultivated in Pakistan. Low moisture content has been reported to be beneficial for shelf life, as it minimizes microbial activity and spoilage, thereby enhancing storability (Belyaeva et al., 2022). The low moisture content and favorable storability characteristics make YMB a resilient food commodity that can be safely stored for extended periods. This enhances their utility as a buffer food during lean seasons or supply disruptions.
Ash content, indicative of the total mineral composition, was measured at 3.49 g/100 g. This result closely aligns with that of Zafar et al. (2023), who reported an ash content of 3.67 g/100 g, and falls within the range of 2.78-3.53 g/100 g observed by Wang et al. (2021) in 24 mung bean genotypes from China.
The crude protein content of 23.07 g/100 g underscores the nutritional significance of mung beans as a plant-based protein source. This high protein level makes them particularly suitable for vegetarian and vegan diets, as well as for populations with limited access to animal-derived proteins. The value obtained is within the range reported by Wang et al. (2021) (17.36-24.89 g/100 g) and is comparable to the findings of Idris et al. (2025), who observed protein contents between 22.63 and 25.84 g/100 g. Protein also contributes significantly to the total caloric value of mung beans.
Crude fat content was found to be 2.09 g/100 g, which is relatively low and consistent with the typical lipid profile of legumes. This value is marginally higher than that reported by Idris et al. (2025) (1.13-1.63 g/100 g), but considerably lower than the range reported by Wang et al. (2021) (4.24-12.18 mg/g). The low-fat content enhances the desirability of mung beans for low-fat dietary regimens. Despite the low-fat levels, mung beans have been reported to contain essential fatty acids beneficial to health (Słowik-Borowiec et al., 2022).
Carbohydrates, calculated by difference, constituted the major macronutrient at 63.86 g/100 g. This value is higher than those reported by Idris et al. (2025) (54.90-58.82 g/100 g) and by Widjajaseputra et al. (2019) for Indonesian mung beans. Carbohydrates are a primary source of dietary energy.
The total energy value was 366.52 kcal/100 g, reflecting the integrated caloric contribution of proteins, carbohydrates, and fats. This value is slightly higher than the 333.0 kcal/100 g reported by Masood et al. (2014), likely due to the comparatively higher protein and carbohydrate contents in the present sample. The energy density of mung beans reinforces their role in addressing caloric requirements, particularly in regions facing nutritional insecurity.
Taken together, the high protein content, minimal fat, and substantial energy value position YMB as a valuable staple for improving diet quality, particularly among low-income or predominantly plant-based populations.
The total mineral content of YMB presented in Table 2 reveals a mineral-rich profile, making them a valuable dietary component, particularly in plant-based diets. Every mineral is essential for human nutrition, and the analyzed concentrations offer valuable information regarding the health benefits associated with YMB consumption.
| Mineral | Result (mg/100 g) |
|---|---|
| Potassium | 1,290.29 ± 2.411) |
| Magnesium | 157.52 ± 1.38 |
| Calcium | 70.50 ± 0.31 |
| Iron | 3.57 ± 0.06 |
| Sodium | 3.00 ± 0.07 |
| Zinc | 2.44 ± 0.05 |
| Manganese | 1.01 ± 0.02 |
| Copper | 0.90 ± 0.00 |
Among the macrominerals, potassium was found at a remarkably high level of 1,290.29 mg/100 g, underscoring the potential of mung beans to contribute significantly to daily potassium requirements. This value falls within the range of 867 to 1,410 mg/100 g reported by Nair et al. (2015) for mung bean seeds grown in India. This mineral plays a vital role in supporting heart health, regulating fluid balance, and ensuring proper nerve signal transmission (Kowey, 2002). It also supports bone health and is associated with a reduced risk of stroke and coronary heart disease (Weaver, 2013).
Magnesium content was also considerable at 157.52 mg/100 g, aligning with the range reported by Nair et al. (2015), which was 143 to 170 mg/100 g. Magnesium is recognized as a cofactor in over 300 enzymatic-catalyzed reactions and plays both therapeutic and preventive roles in chronic conditions, for instance, diabetes and cardiovascular disease (Al Alawi et al., 2018; Gröber et al., 2015).
Calcium was present at 70.50 mg/100 g, which is lower than the levels reported by Nair et al. (2015) and Dahiya et al. (2013), ranging from 119 to 158 mg/100 g and 81 to 114 mg/100 g, respectively. Although lower than dairy sources, this level still makes a meaningful contribution to daily calcium intake, particularly for lactose-intolerant individuals or those following plant-based diets. Calcium is vital for bone health, fluid balance, blood clotting, blood pressure regulation, enzyme activation, muscle contraction, and nerve transmission (Marcus, 2013).
Among the microminerals, iron was the most abundant, measured at 3.57 mg/100 g, which is on the lower end of the 3.5 to 8.7 mg/100 g range reported by Nair et al. (2015). Iron is critical for oxygen transport and energy metabolism (Hirota, 2019; Kim et al., 2022).
Zinc (2.44 mg/100 g) and copper (0.90 mg/100 g) were also present in notable amounts. The zinc content falls on the lower end of the range reported by Nair et al. (2015) (2.1-6.2 mg/100 g) and is slightly below the range provided by Zafar et al. (2023) (2.47-3.72 mg/100 g). In contrast, the copper content is higher than that reported by Zafar et al. (2023) (0.23-0.88 mg/100 g). Zinc is essential for immune function, enzyme activity, and wound healing (Lin et al., 2017), while copper plays vital roles in iron metabolism and cardiovascular health (Kondaiah et al., 2019; Liu and Miao, 2022).
Manganese, at 1.01 mg/100 g, contributes to normal growth, antioxidant defense, and bone health (Tseng et al., 2025), and is consistent with the range reported by Nair et al. (2015), which was 0.98 to 1.96 mg/100 g.
Sodium, measured at only 3.00 mg/100 g, was notably lower than the range reported by Nair et al. (2015), which varied from 11.1 to 13.4 mg/100 g. This low sodium content is advantageous for reducing overall dietary sodium intake. As such, mung beans represent a healthy food option, particularly suitable for individuals seeking to manage blood pressure or lower their risk of cardiovascular disease.
The mineral profile of YMB highlights its value as a nutrient-dense legume capable of helping address dietary micronutrient gaps. With substantial levels of both macro- and microminerals, YMB can contribute meaningfully to daily mineral requirements even in modest serving sizes, making it particularly beneficial for populations with limited access to diverse or mineral-rich foods. The diversity and density of minerals further position YMB as a strategic crop for enhancing nutrient adequacy at household and community levels. Its capacity to provide multiple essential minerals in a single, shelf-stable, and affordable food item supports efforts to reduce macro- and micronutrient deficiencies, especially in resource-constrained settings.
Table 3 presents the percent contribution of 100 g of YMB to the recommended daily nutrient intake for adults aged 19-29 years, based on the EAR or AI values from the PDRI 2015 (DOST-FNRI, 2017). The analysis highlights YMB’s potential to address both protein and several key macro and micromineral needs, particularly in adults.
As detailed in Table 3, YMB is an accessible plant-based protein source and is rich in essential minerals, fulfilling a majority of the daily requirements for zinc, magnesium, and potassium for both male and females. The nutritional contribution of YMB exhibits notable differences between males and females, primarily reflecting variations in recommended daily requirements. For nutrients such as protein, zinc, and magnesium, YMB provides a higher proportion of daily needs for females, as their requirements are lower than those of males.
Conversely, for iron, females receive a smaller fraction of their daily requirement due to their higher physiological needs, particularly women of reproductive age who experience greater iron losses through menstruation (Dugan et al., 2024). Contributions of calcium, potassium, and sodium are similar for both sexes, as their recommended intakes are equivalent. These trends suggest that YMB can play a significant role in improving nutrient adequacy for both adult males and females, although additional iron-rich foods may be necessary to meet the higher iron requirements in women. Meanwhile, the low sodium content of YMB represents an advantage contributing to less than 1% of the recommended limit, this aligns perfectly with the PDRI 2015 guideline to limit the sodium intake to less than 2,000 mg per day (DOST-FNRI, 2017), making YMB an ideal functional food for managing cardiovascular health and hypertension.
While the mineral profile of YMB has a high potential due to its nutrient content, it is also worth noting that its actual bioavailability may be affected by inherent antinutritional factors. Compounds like phytates and tannins can bind to essential minerals like iron, zinc, and calcium, thereby inhibiting their mineral absorption (Hou et al., 2019; Sudkaharan and Bukkan, 2021). Moreover, food processing techniques like soaking, sprouting, and cooking have been shown to effectively degrade these anti-nutritional compounds and significantly improve mineral bioaccessibility (Elobuike et al., 2021; Wanaina et al., 2021). Furthermore, these findings highlight the potential of locally grown YMB to contribute to the dietary needs of Filipinos, providing evidence to encourage consumers, farmers, and the food industry to prioritize local varieties over imported legumes.
The amino acid composition of YMB is summarized in Fig. 1. The amino acid composition of YMB, excluding tryptophan due to analytical limitations, reveals a balanced composition of both indispensable and dispensable amino acids, comprising 40.12% and 59.88% of the total amino acid content, respectively. This distribution suggests that while YMB is a particularly rich source of dispensable amino acids, it also provides a substantial proportion of non-dispensable amino acids, vital for human health and must be obtained through the diet.
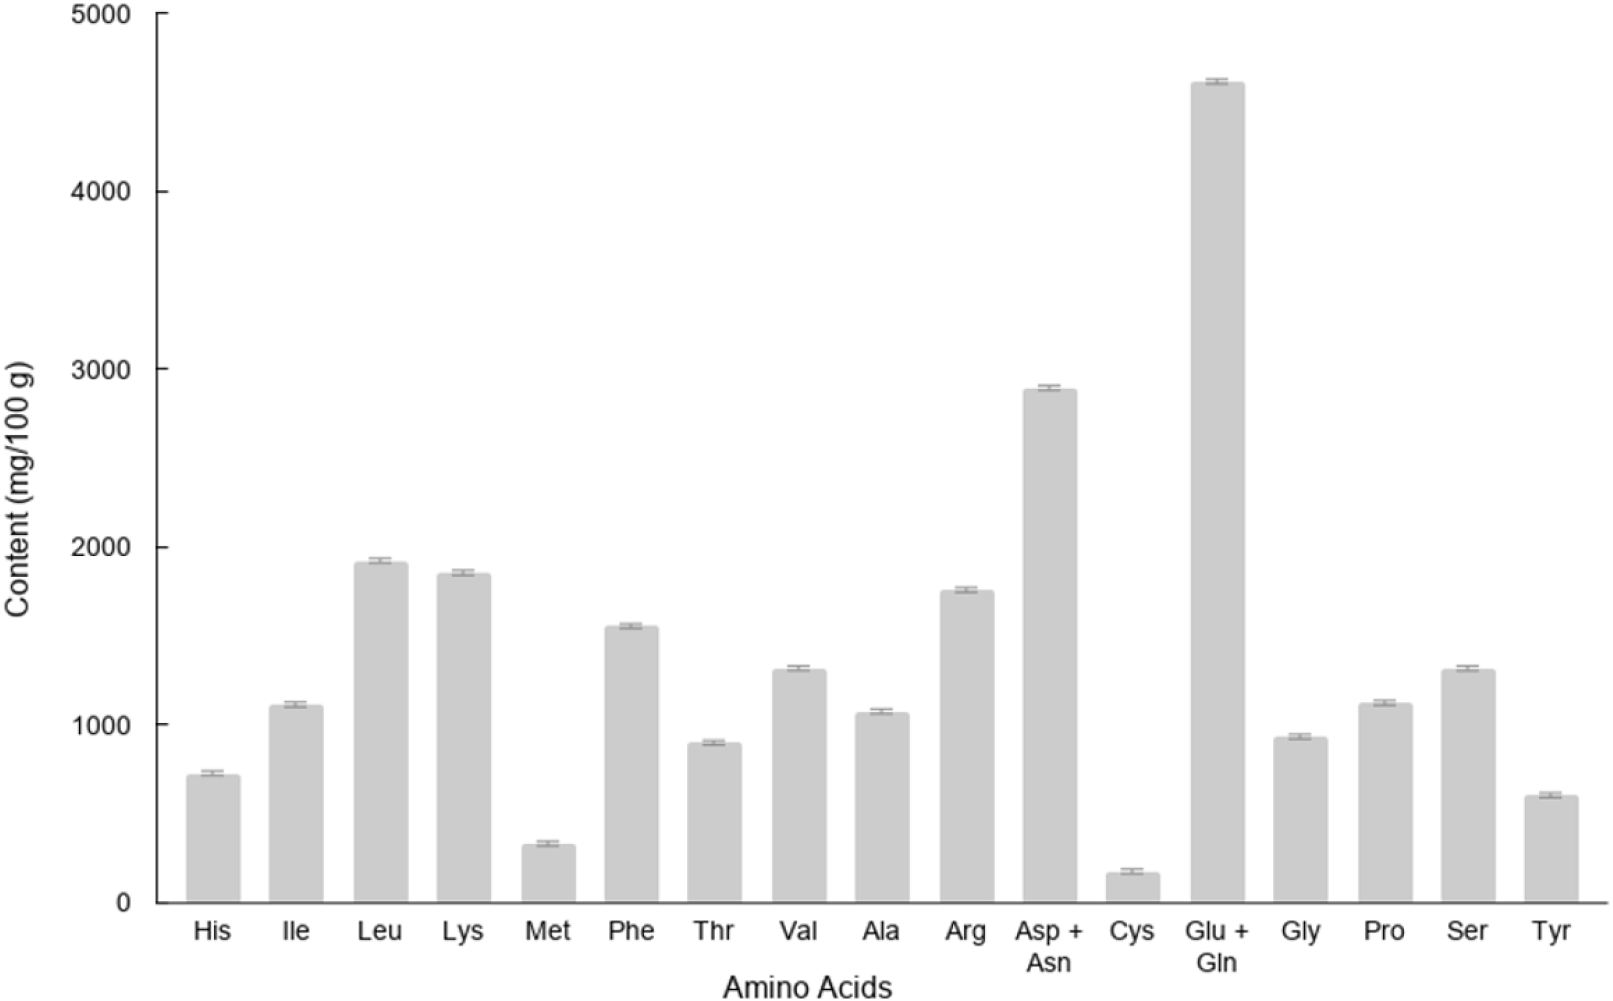
Among the eight non-dispensable amino acids evaluated, the branched-chain amino acids leucine (1,922 mg/100 g), valine (1,317 mg/100 g) and isoleucine (1,113 mg/100 g) showed relatively high concentrations, contributing to the branched-chain amino acid (BCAA) profile important for protein synthesis and turnover as well as maintenance of the body glutamate-glutamine level (Tamanna and Mahmood, 2014).
Lysine (1,854 mg/100 g) was found to be the second most abundant non-dispensable amino acid. This is particularly notable because lysine is often a limiting amino acid in cereal-based diets, indicating that YMB could play a key role in improving protein quality when consumed in combination with grains (Boye et al., 2010).
Phenylalanine (1,554 mg/100 g) and threonine (898 mg/100 g) further enhanced the YMB’s amino acid profile, supporting its use in the synthesis of other proteins. On the lower end, histidine (727 mg/100 g) and methionine (331 mg/100 g) were present in lesser amounts. Methionine, a sulfur-containing amino acid, is typically limited in legumes, and this trend is evident here. This suggests the need to complement mung legume-based diets with methionine-rich foods for balanced protein intake.
Among the dispensable amino acids, the combined levels of glutamic acid and glutamine were the most abundant, with a concentration of 4,615 mg/100 g, followed by the combined levels of aspartic acid and asparagine at 2,893 mg/100 g. Glutamic acid and glutamine are known for their roles in amino acid metabolism and nitrogen regulation in the body (Kulkarni et al., 2005). Aspartic acid, like glutamic acid, functions as an excitatory neurotransmitter, facilitating signal transmission between neurons (Dingledine and McBain, 1999) underscoring their physiological importance beyond protein synthesis. Asparagine, an amide derivative of aspartic acid, is involved in protein synthesis and N-glycosylation (Safrhansova et al., 2022).
At 1,757 mg/100 g, arginine was the third highest among the dispensable amino acids, highlighting its role in multiple biological processes, including its catabolism into intermediates that replenish components of the Krebs cycle (Albaugh and Barbul, 2017a). Serine and proline were also present in significant amounts—1,317 mg/100 g and 1,122 mg/100 g, respectively. Beyond its involvement in protein synthesis, serine is essential for neurotransmission and participates in the folate and methionine cycles, as well as in the biosynthesis of sphingolipids, phospholipids, and sulfur-containing amino acids (Holeček, 2022). Proline, meanwhile, plays a critical role in collagen synthesis and maintaining structural integrity of proteins (Albaugh et al., 2017).
Alanine (1,075 mg/100 g) and glycine (933 mg/100 g) were found at moderate concentrations, both of which contribute to cellular protection mechanisms, particularly in safeguarding kidney cells from stress-induced damage (Nissim et al., 1992). Tyrosine, the least abundant among the principal dispensable amino acids at 603 mg/100 g, serves as a precursor for several critical hormones and catecholamine neurotransmitters (Moon et al., 2018). Cystine, reported as the combined value of cystine and cysteine and expressed as cystine, had the lowest concentration at 176 mg/100 g. Despite its lower abundance, cystine plays a crucial role in forming disulfide bonds that stabilize protein structure and functions as a key precursor in glutathione synthesis, a major antioxidant in the body (Yu and Long, 2016).
The YMB seeds exhibited the following phytochemicals and antioxidant activity as indicated in Table 4.
| Assay1) | Result |
|---|---|
| TPC (mg GAE/100 g DW) | 53.68 ± 2.722) |
| DPPH (μmol TE/100 g DW) | 21.32 ± 0.07 |
| FRAP (μmol TE/100 g DW) | 42.16 ± 0.64 |
The TPC of YMB (53.68 mg GAE/100 g DW) obtained in this study is lower than those reported by Yusnawan et al. (2019), who assessed 14 mung bean cultivars from Indonesia and falls within the lower range of values reported by Parikh and Patel (2018) for Indian pulses, which varied from 38.6 to 542.7 mg GAE/100 g DW. Variations in solvent type, extraction time, temperature, and other processing parameters can significantly influence the measured values, which may partly explain the discrepancies among studies. It should also be noted that the TPC measured in this study reflects only the phenolic compounds extractable under the specific experimental conditions and does not represent the total phenolic content of the whole sample or its activity in vivo. Phenolic compounds are widely recognized for their strong antioxidant activity, primarily attributed to their capacity to neutralize free radicals and bind metal ions. Through these mechanisms, they help alleviate oxidative stress, which is linked to a decreased risk of developing chronic illnesses such as cardiovascular disease, certain cancers, and neurodegenerative disorders (Sun et al., 2014).
Antioxidant activity was further assessed using the DPPH and FRAP assays. The DPPH radical scavenging capacity of YMB was found to be 21.32 μmol TE/100 g DW, while its FRAP was 42.16 μmol TE/100 g DW. These values are considerably lower than those reported by Priti et al. (2021) across 20 diverse genotypes of mung beans and lentils, which ranged from 69.00 to 158.50 μmol TE/100 g for DPPH and 570.00 to 1,130.00 μmol TE/100 g for FRAP. Differences in antioxidant activity across studies may be attributed to variation in genotype, sample preparation, and analytical methods.
Polyphenols have been reported to interact with macronutrients and micronutrients in various ways (Cianciosi et al., 2022). These interactions may include associations with lipids, proteins, carbohydrate digestibility, and mineral complex formation. Such effects have been described in the literature in relation to nutrient bioavailability and food matrix interactions.
The low values in all three indicate that the YMB used in this study has less capacity to neutralize oxidative stress, meaning it provides fewer antioxidant benefits compared to cultivars with higher TPC and radical-scavenging activity. However, these results may actually be favorable for mineral absorption, as there would be fewer polyphenol-mineral complexes that inhibit uptake.
4. Conclusions
This study was limited to a single mung bean variety, and the sample was collected from only one farming season, which may affect the generalizability of the results. Future research could expand on these findings by evaluating multiple mung bean cultivars across different growing seasons. Additionally, further studies are recommended to assess mineral bioavailability, protein quality, and other anti-nutritional factors such as tannins and phytates to provide a more comprehensive understanding of the nutritional potential of mung beans.
The locally grown YMB used in this study are high in protein, amino acids, and essential minerals. The ethanolic extract exhibited a lower concentration of phenolic compounds and antioxidant activities when compared to other studied mung beans. This study further underscores its nutritional significance, as 100 g can supply a substantial portion of the daily mineral requirements for Filipino adults. Given the nutritional density of YMB and their adaptability to local farming conditions, promoting the cultivation and consumption of locally grown mung beans could help reduce the Philippines’ dependence on imports, strengthen food security, and promote sustainable agriculture.